EP0736099B1 - Expression of self-processing polyproteins in transgenic plants - Google Patents
Expression of self-processing polyproteins in transgenic plants Download PDFInfo
- Publication number
- EP0736099B1 EP0736099B1 EP95903855A EP95903855A EP0736099B1 EP 0736099 B1 EP0736099 B1 EP 0736099B1 EP 95903855 A EP95903855 A EP 95903855A EP 95903855 A EP95903855 A EP 95903855A EP 0736099 B1 EP0736099 B1 EP 0736099B1
- Authority
- EP
- European Patent Office
- Prior art keywords
- sequence
- protein
- translation
- polyprotein
- cleavage site
- Prior art date
- Legal status (The legal status is an assumption and is not a legal conclusion. Google has not performed a legal analysis and makes no representation as to the accuracy of the status listed.)
- Expired - Lifetime
Links
Images


Classifications
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K14/00—Peptides having more than 20 amino acids; Gastrins; Somatostatins; Melanotropins; Derivatives thereof
- C07K14/005—Peptides having more than 20 amino acids; Gastrins; Somatostatins; Melanotropins; Derivatives thereof from viruses
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N15/00—Mutation or genetic engineering; DNA or RNA concerning genetic engineering, vectors, e.g. plasmids, or their isolation, preparation or purification; Use of hosts therefor
- C12N15/09—Recombinant DNA-technology
- C12N15/11—DNA or RNA fragments; Modified forms thereof; Non-coding nucleic acids having a biological activity
- C12N15/62—DNA sequences coding for fusion proteins
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N15/00—Mutation or genetic engineering; DNA or RNA concerning genetic engineering, vectors, e.g. plasmids, or their isolation, preparation or purification; Use of hosts therefor
- C12N15/09—Recombinant DNA-technology
- C12N15/63—Introduction of foreign genetic material using vectors; Vectors; Use of hosts therefor; Regulation of expression
- C12N15/79—Vectors or expression systems specially adapted for eukaryotic hosts
- C12N15/82—Vectors or expression systems specially adapted for eukaryotic hosts for plant cells, e.g. plant artificial chromosomes (PACs)
- C12N15/8216—Methods for controlling, regulating or enhancing expression of transgenes in plant cells
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N15/00—Mutation or genetic engineering; DNA or RNA concerning genetic engineering, vectors, e.g. plasmids, or their isolation, preparation or purification; Use of hosts therefor
- C12N15/09—Recombinant DNA-technology
- C12N15/63—Introduction of foreign genetic material using vectors; Vectors; Use of hosts therefor; Regulation of expression
- C12N15/79—Vectors or expression systems specially adapted for eukaryotic hosts
- C12N15/82—Vectors or expression systems specially adapted for eukaryotic hosts for plant cells, e.g. plant artificial chromosomes (PACs)
- C12N15/8241—Phenotypically and genetically modified plants via recombinant DNA technology
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N9/00—Enzymes; Proenzymes; Compositions thereof; Processes for preparing, activating, inhibiting, separating or purifying enzymes
- C12N9/14—Hydrolases (3)
- C12N9/48—Hydrolases (3) acting on peptide bonds (3.4)
- C12N9/50—Proteinases, e.g. Endopeptidases (3.4.21-3.4.25)
- C12N9/503—Proteinases, e.g. Endopeptidases (3.4.21-3.4.25) derived from viruses
- C12N9/506—Proteinases, e.g. Endopeptidases (3.4.21-3.4.25) derived from viruses derived from RNA viruses
-
- C—CHEMISTRY; METALLURGY
- C07—ORGANIC CHEMISTRY
- C07K—PEPTIDES
- C07K2319/00—Fusion polypeptide
- C07K2319/61—Fusion polypeptide containing an enzyme fusion for detection (lacZ, luciferase)
-
- C—CHEMISTRY; METALLURGY
- C12—BIOCHEMISTRY; BEER; SPIRITS; WINE; VINEGAR; MICROBIOLOGY; ENZYMOLOGY; MUTATION OR GENETIC ENGINEERING
- C12N—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA
- C12N2770/00—MICROORGANISMS OR ENZYMES; COMPOSITIONS THEREOF; PROPAGATING, PRESERVING, OR MAINTAINING MICROORGANISMS; MUTATION OR GENETIC ENGINEERING; CULTURE MEDIA ssRNA viruses positive-sense
- C12N2770/00011—Details
- C12N2770/36011—Togaviridae
- C12N2770/36111—Alphavirus, e.g. Sindbis virus, VEE, EEE, WEE, Semliki
- C12N2770/36122—New viral proteins or individual genes, new structural or functional aspects of known viral proteins or genes
Definitions
- This invention relates generally to the expression of self-processing polyproteins in transgenic plants.
- the relative levels of expression of several introduced genes in transgenic plants is notoriously influenced by "position effects" determined by the particular site of transgene integration into the genome. Even when introduced genes are linked on the same T-DNA, driven either by convergent or divergent promoters, they are usually not co-ordinately expressed at similar levels. This poses particular problems when high levels of expression of a number of introduced activities is required, for instance when attempting to express novel biochemical pathways in plants. In an attempt to achieve tissue specific, co-ordinated expression of two proteins, other researchers have linked genes by co-transference on the same T-DNA.
- Linking proteins in the form of polyproteins is a strategy adopted in the replication of many viruses.
- virus-encoded proteinases mediate extremely rapid intramolecular (cis) cleavages of the polyprotein to yield discrete protein products.
- a number of viral proteinases have been partially characterised and are thought to be related, both structurally and in catalytic mechanism, to cellular proteinases.
- picornaviridae a single long open reading frame encodes a polyprotein of some 225kD, but full-length translation products are not normally observed due to extremely rapid "primary" intramolecular (cis) cleavages mediated by virus encoded proteinases.
- cis intramolecular
- a primary cleavage occurs between the P1 capsid protein precursor and the replicative domains of the polyprotein (P2, P3; Figure 1,A). This cleavage is mediated by a virus encoded proteinase (2A pro ), of some 17kDa, cleaving at its own N-terminus.
- FMDV polyprotein undergoes a primary polyprotein cleavage at the C-terminus of the 2A region between the capsid protein precursor (P1-2A) and replicative domains of the polyprotein 2BC and P3 ( Figure 1,B). Precursors spanning the 2A/2B cleavage site are not detected during native polyprotein processing. This situation is somewhat analogous to the 2A cleavage in entero- and rhinoviruses described above. However the 2A region of the FMDV polyprotein was demonstrated to be only 16 amino acids long (Figure 1,C).
- the predicted amino acid sequence of this region is totally conserved amongst all aphthovirus genomic RNAs sequenced to date.
- the FMDV 2A region also shows high similarity to the C-terminal region of the approximately ten fold larger 2A protein of another genus of the picornaviridae, the cardioviruses.
- a method for the expression of multiple proteins in a transgenic plant comprising inserting into the genome of the plant a gene construct comprising a 5'-region which includes a promoter which is capable of initiating transcription of a structural gene under the control thereof, a protein encoding sequence coding for more than one protein and a 3'-terminator region which includes a polyadenylation signal, each of the said protein encoding sequences being separated from an adjacent protein encoding sequence by a DNA LINKER sequence which on translation autoproteolytically cleaves to give the component protein molecules.
- the DNA sequence which encodes the post-translation cleavage site is derived from a virus, particularly a picornavirus.
- the DNA sequence providing the cleavage site encodes the amino acid sequence NFDLLKLAGDVESNPGPFF [SEQ ID NO.1].
- the amino acid sequence NFDLLKLAGDVESNPGPFF amino acid sequence NFDLLKLAGDVESNPGPFF [SEQ ID NO.1].
- FMDV 2A represents a polyprotein region whose sole function in the viral genome is to effect or direct a single cleavage at its own C-terminus, functioning only in cis. Due to its small size, FMDV 2A (and related sequences or derivatives) presents an ideal candidate for engineering into plant polyprotein expression vectors.
- FMDV 2A functions as a substrate for a cellular proteinase, which, to account for the observed cleavage kinetics, would need to be closely coupled to translation, (ii) the FMDV 2A sequence in some manner disrupts the normal peptide bond formation during translation, or (iii) the FMD 2A sequence possesses an entirely novel type of proteolytic activity.
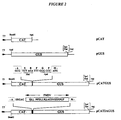
- pCAT2AGUS plasmid in which the 20 amino acid sequence spanning FMDV 2A was inserted between the reporter genes chloramphenicol acetyl transferase (CAT) and ß-glucuronidase (GUS) maintaining a single, long, open reading frame ( Figure 2).
- CAT chloramphenicol acetyl transferase
- GUS ß-glucuronidase
- Figure 2 a plasmid
- FMDV sequence can function in a manner similar to that observed in FMDV polyprotein processing: the [CAT2AGUS] polyprotein undergoes a co-translational, apparently autoproteolytic, cleavage yielding [CAT-2A] and GUS. It is clear that the 20 amino acid FMDV 2A-spanning sequence does not require other domains within the FMDV polyprotein to function and is an autonomous element capable of mediating cleavage-even in a completely foreign context.
- an oligopeptide comprising the C-terminal 14 residues of the EMC 2A protein together with the N-terminal proline residue of EMC protein 2B can also mediate cleavage in a foreign context, although to a lower level than FMD 2A
- FMDV 2A together with the N-terminal proline residue of protein 2B may represent an entirely novel type of protein cleavage activity. Although the mechanism of cleavage is not yet understood, its utility is apparent. Because of its small size the FMDV 2A sequence or derivatives of it are particularly attractive candidates for use in plant polyprotein expression constructs enabling the co-ordinated and stoichiometric expression of multiple proteins from a single open reading frame.
- the FMDV 2A sequence (plus the requisite carboxy-terminal proline) inserted between protein coding sequences, may allow the engineering of plant expression vectors where multiple whole proteins or protein domains can be expressed as a polyprotein and cleaved apart co-translationally with high efficiency. This may enable the rapid introduction of entire enzyme cascades into plants.
- the reporter genes CAT and GUS were amplified by PCR using oligonucleotide primers such that restriction sites were created at both termini.
- Individual genes were cloned into pGEM transcription vectors (pCAT; pGUS) and also assembled together (pCATGUS) to produce a single open reading frame encoding the artificial polyprotein [CATGUS] ( Figure 2).
- Coding sequences from the FMDV 2A region were assembled in the plasmid vector pGEM 7zf(+) in such a way that a series of unique restriction sites were created throughout the sequence.
- the FMDV 2A sequence was excised and inserted between the CAT and GUS genes of pCATGUS to retain a single open reading frame and form construct pCAT2AGUS ( Figure 2).
- Translation studies were performed in a coupled transcription/ translation (TnT) wheat germ system using T7 polymerase.
- Translation directed by plasmids pCAT , pGUS and pCATGUS yielded polypeptides of the expected molecular weight for CAT (25.7kDa), GUS (70.4kDa) and the polyprotein [CATGUS] (96.3kDa) respectively ( Figure 3, lanes 1, 4 and 2).
- Translation directed by pCAT2AGUS yielded two major products at 70kDa and 26kDa (lane 3). The 70kDa polypeptide migrated identically to the product of pGUS shown in lane 1 and represents GUS polypeptide processed from the [CAT2AGUS] polyprotein during translation.
- the 26kDa band migrated slightly more slowly than the product of pCAT shown in lane 4 and corresponds to the [CAT-2A] cleavage product.
- a third fainter band appeared at approx. 96kDa (lane 3) and co-migrated with the product of pCATGUS (lane 2). This corresponds to the entire polyprotein product of pCAT2AGUS and suggests that a small proportion of the polyprotein is not processed in the wheat germ lysate.
- Densitometric analysis of the distribution of radiolabel in the polypeptides in lane 3 showed that over 90% of the [CAT2AGUS] translation product was cleaved to [CAT-2A] and GUS.
- the [CAT2AGUS] portion of pCAT2AGUS was excised, inserted between the 35S CaMV promoter and nos 3' terminator and cloned into a Binl9-derived plant expression vector containing a functional neomycin phosphotransferase gene.
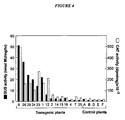
- This construct was introduced into tobacco via Agrobacterium- mediated leaf disk transformation. Transformed plants were selected and rooted on kanamycin. Protein extracts were prepared from leaves of transformed plants and assayed for GUS and CAT activities. The results are shown in Figure 4. A high degree of correlation was found between the activities of the two enzymes in any given plant. Of 18 independent transformed plants, seven plants (6, 26, 28, 24, 29, 1 and 12) expressed both enzymes at relatively high levels. Four plants (2, 14, 15, 16) expressed both enzymes at low levels. The remaining plants (only three shown in Figure 4, plants 4, 7 and 25) did not express either enzyme at levels above that detected in untransformed control plants (A, B, D, E, F).
- the data presented here demonstrates that the FMDV 2A sequence can function in a manner similar to that observed in FMDV polyprotein processing when expressed in chimeric genes in plant extracts and cells. Both in wheat germ lysates and transgenic plants, the chimeric [CAT2AGUS] polyprotein undergoes rapid, apparently autoproteolytic, cleavage to yield [CAT-2A] and GUS.
- FMDV 2A may represent an entirely novel type of protein cleavage activity. Although the mechanism of cleavage is not yet understood, its utility is apparent. Because of it's small size the FMDV 2A sequence or derivatives of it are particularly attractive candidates for use in plant polyprotein expression constructs enabling the coordinated and stoichiometric expression of multiple proteins from a single open reading frame.
- the FMDV 2A sequence inserted between protein coding sequences allows the engineering of plant expression vectors where multiple whole proteins or protein domains can be expressed as a polyprotein and cleaved apart co-translationally with high efficiency. This may enable the rapid introduction of entire enzyme cascades into plants.
Landscapes
- Health & Medical Sciences (AREA)
- Life Sciences & Earth Sciences (AREA)
- Genetics & Genomics (AREA)
- Chemical & Material Sciences (AREA)
- Engineering & Computer Science (AREA)
- Organic Chemistry (AREA)
- Molecular Biology (AREA)
- Biomedical Technology (AREA)
- Bioinformatics & Cheminformatics (AREA)
- Wood Science & Technology (AREA)
- Zoology (AREA)
- Biotechnology (AREA)
- General Engineering & Computer Science (AREA)
- General Health & Medical Sciences (AREA)
- Biochemistry (AREA)
- Biophysics (AREA)
- Microbiology (AREA)
- Plant Pathology (AREA)
- Physics & Mathematics (AREA)
- Virology (AREA)
- Medicinal Chemistry (AREA)
- Cell Biology (AREA)
- Gastroenterology & Hepatology (AREA)
- Proteomics, Peptides & Aminoacids (AREA)
- Breeding Of Plants And Reproduction By Means Of Culturing (AREA)
- Micro-Organisms Or Cultivation Processes Thereof (AREA)
- Cultivation Of Plants (AREA)
- Compounds Of Unknown Constitution (AREA)
- Agricultural Chemicals And Associated Chemicals (AREA)
- Enzymes And Modification Thereof (AREA)
- Peptides Or Proteins (AREA)
Abstract
Description
- This invention relates generally to the expression of self-processing polyproteins in transgenic plants.
- The relative levels of expression of several introduced genes in transgenic plants is notoriously influenced by "position effects" determined by the particular site of transgene integration into the genome. Even when introduced genes are linked on the same T-DNA, driven either by convergent or divergent promoters, they are usually not co-ordinately expressed at similar levels. This poses particular problems when high levels of expression of a number of introduced activities is required, for instance when attempting to express novel biochemical pathways in plants. In an attempt to achieve tissue specific, co-ordinated expression of two proteins, other researchers have linked genes by co-transference on the same T-DNA. The expression levels of linked nopaline synthase (nos) and octopine synthase (ocs) genes and closely adjacent neomycin phosphotransferase II (NPTII) and chloramphenicol acetyl transferase (CAT) reporter genes were found to vary independently. Another strategy was to link genes via adjacent and divergent promoters. Whereas co-ordinated expression of the Cab22L and Cab22R genes of petunia was achieved, a similar approach using the CAT and GUS genes produced a high degree of variation of CAT and GUS activities within individual transgenes.
- Linking proteins in the form of polyproteins is a strategy adopted in the replication of many viruses. On translation, virus-encoded proteinases mediate extremely rapid intramolecular (cis) cleavages of the polyprotein to yield discrete protein products.
- A number of viral proteinases have been partially characterised and are thought to be related, both structurally and in catalytic mechanism, to cellular proteinases. In the picornaviridae a single long open reading frame encodes a polyprotein of some 225kD, but full-length translation products are not normally observed due to extremely rapid "primary" intramolecular (cis) cleavages mediated by virus encoded proteinases. In the case of the entero- and rhinoviruses, a primary cleavage occurs between the P1 capsid protein precursor and the replicative domains of the polyprotein (P2, P3; Figure 1,A). This cleavage is mediated by a virus encoded proteinase (2Apro), of some 17kDa, cleaving at its own N-terminus.
- The aphtho-, or Foot-and-Mouth Disease (FMD), viruses form a distinct group within the picornaviridae. FMDV polyprotein undergoes a primary polyprotein cleavage at the C-terminus of the 2A region between the capsid protein precursor (P1-2A) and replicative domains of the polyprotein 2BC and P3 (Figure 1,B). Precursors spanning the 2A/2B cleavage site are not detected during native polyprotein processing. This situation is somewhat analogous to the 2A cleavage in entero- and rhinoviruses described above. However the 2A region of the FMDV polyprotein was demonstrated to be only 16 amino acids long (Figure 1,C). The predicted amino acid sequence of this region, is totally conserved amongst all aphthovirus genomic RNAs sequenced to date. The FMDV 2A region also shows high similarity to the C-terminal region of the approximately ten fold larger 2A protein of another genus of the picornaviridae, the cardioviruses.
- According to the present invention, there is provided a method for the expression of multiple proteins in a transgenic plant comprising inserting into the genome of the plant a gene construct comprising a 5'-region which includes a promoter which is capable of initiating transcription of a structural gene under the control thereof, a protein encoding sequence coding for more than one protein and a 3'-terminator region which includes a polyadenylation signal, each of the said protein encoding sequences being separated from an adjacent protein encoding sequence by a DNA LINKER sequence which on translation autoproteolytically cleaves to give the component protein molecules.
- Preferably the DNA sequence which encodes the post-translation cleavage site is derived from a virus, particularly a picornavirus.
- Preferably also the DNA sequence providing the cleavage site encodes the amino acid sequence NFDLLKLAGDVESNPGPFF [SEQ ID NO.1]. However, it is well known that variations may be made in amino acid sequences which do not greatly affect function and it is intended that such variants of the said sequence and the nucleotide which encodes it are within the scope of this invention.
- Thus multiple genes are inserted into a plant genome under the control of a single promoter, in the form of a self-processing polyprotein.
- We have found that
FMDV 2A represents a polyprotein region whose sole function in the viral genome is to effect or direct a single cleavage at its own C-terminus, functioning only in cis. Due to its small size,FMDV 2A (and related sequences or derivatives) presents an ideal candidate for engineering into plant polyprotein expression vectors. - The inclusion of such proteinase or cleavage sequences in plant transformation constructs enables the expression from a single promoter of multiple introduced proteins, initially linked as a polyprotein, in plant cells and plants.
- Initial characterisation of the
FMDV 2A region, using a series of recombinant FMDV polyproteins, showed that theFMDV 2A/2B cleavage activity was mediated by residues located within the 19 amino acid sequence NFDLLKLAGDVESNPGPFF [SEQ ID NO. 1] spanning the FMDV 2A region (Ryan et al, 1991). It was found that FMDV 2A does not act as a substrate for a proteinase located elsewhere within the FMDV polyprotein or absolutely require particular FMDV domains for activity. Three explanations may account for a co-translational cleavage associated with such a short sequence; (i)FMDV 2A functions as a substrate for a cellular proteinase, which, to account for the observed cleavage kinetics, would need to be closely coupled to translation, (ii) theFMDV 2A sequence in some manner disrupts the normal peptide bond formation during translation, or (iii) theFMD 2A sequence possesses an entirely novel type of proteolytic activity. These data do not, however, clarify to what extent the 2A region could function independently of the physical environment provided by FMDV polyprotein sequences. To address this question we have studied proteolysis associated withFMDV 2A in a completely foreign context, that of a synthetic polyprotein designed such that two reporter genes flank sequences from theFMDV 2A region of the polyprotein. - We have constructed a plasmid (pCAT2AGUS) in which the 20 amino acid
sequence spanning FMDV 2A was inserted between the reporter genes chloramphenicol acetyl transferase (CAT) and ß-glucuronidase (GUS) maintaining a single, long, open reading frame (Figure 2). Translation studies were performed in three systems; (i) a coupled transcription / translation (TnT) rabbit reticulocyte system, (ii) a wheat germ lysate and (iii) a human cell line (HTK-143) infected with the recombinant vaccinia virus vTF7-3 expressing T7 RNA polymerase. - Translation directed by pCAT2AGUS showed three major translation products in all translation systems. The uppermost band corresponded to the expected [CAT2AGUS] polyprotein translation product and was immunoprecipitated by anti-CAT and anti-GUS antibodies. The second band co-migrated with GUS and was immunoprecipitated only by antibodies directed against GUS and corresponded to a GUS cleavage product. The lower band migrated somewhat more slowly than CAT and was immunoprecipitated by anti-CAT and anti-2A antibodies but not anti-GUS antibodies and corresponded to the [CAT2A] cleavage product. Densitometric analysis determined that 80% of the translated polyprotein had undergone cleavage to [CAT2A] and [GUS]. Assays provided evidence that both cleaved proteins were enzymically active.
- These analyses show that the inserted FMDV sequence can function in a manner similar to that observed in FMDV polyprotein processing: the [CAT2AGUS] polyprotein undergoes a co-translational, apparently autoproteolytic, cleavage yielding [CAT-2A] and GUS. It is clear that the 20
amino acid FMDV 2A-spanning sequence does not require other domains within the FMDV polyprotein to function and is an autonomous element capable of mediating cleavage-even in a completely foreign context. Our analysis of N-terminally truncated forms ofFMDV 2A show that the 13 residue oligopeptide (-LKLAGDVESNPGP- [SEQ ID NO.2]) is able to mediate cleavage whereas the 11 residue oligopeptide (-LAGDVESNPGP-[SEQ ID NO.3]) is not. However the final proline residue, which comes after the actual 2A cleavage site and constitutes the amino-terminal residue of 2B in FMDV, is necessary for cleavage. In addition we have evidence that an oligopeptide comprising the C-terminal 14 residues of theEMC 2A protein together with the N-terminal proline residue ofEMC protein 2B can also mediate cleavage in a foreign context, although to a lower level thanFMD 2A We are currently determining by mutagenesis the exact amino acid sequences which permit cleavage in an attempt to optimise the reaction. - FMDV 2A together with the N-terminal proline residue of
protein 2B may represent an entirely novel type of protein cleavage activity. Although the mechanism of cleavage is not yet understood, its utility is apparent. Because of its small size theFMDV 2A sequence or derivatives of it are particularly attractive candidates for use in plant polyprotein expression constructs enabling the co-ordinated and stoichiometric expression of multiple proteins from a single open reading frame. - In the model [CAT2AGUS] construct described above, the 20
amino acid 2A-spanning sequence which remains attached to CAT after cleavage from GUS, is sufficiently short that CAT activity is not impaired. We have also found no impairment of activity in similar constructs where 2A is attached to the carboxy terminus of glutathione-S-transferase or T7 RNA polymerase. - We have introduced the CAT2AGUS construct into tobacco plants and will assess the efficiency of cleavage of [CAT2A] from [GUS] in this system. However since the cleavage has been effective in all systems tested to date, including wheatgerm lysates, efficient cleavage is expected. The
FMDV 2A sequence (plus the requisite carboxy-terminal proline) inserted between protein coding sequences, may allow the engineering of plant expression vectors where multiple whole proteins or protein domains can be expressed as a polyprotein and cleaved apart co-translationally with high efficiency. This may enable the rapid introduction of entire enzyme cascades into plants. - The invention will now be described with reference to the accompanying Figures of which:
- Figure 1 shows: Picornavirus Primary Polyprotein
Cleavages. The 5' non-coding region is capped by a small
protein VPg (or 3B). The single long open reading frame
and polyprotein organisation is shown (boxed areas) for
both entero- and rhinovirus groups (panel A) and
aphthoviruses (panel B). Arrows indicate sites of primary
cleavage and the virus-encoded proteinases responsible,
where known. Primary cleavage products are shown below.
The amino acid sequence spanning the
aphthovirus 2A region of the polyprotein is shown, the 2A oligopeptide being cleaved from the capsid protein 1D by 3Cpro in an intermolecular reaction occuring at a later stage of polyprotein processing (panel C); - Figure 2 shows: CAT/GUS Constructs. Boxed areas represent the single open reading frames encoding either individual proteins (CAT; pCAT20/21, GUS; pGUS12/23) or the artificial polyproteins [CATGUS] and [CAT2AGUS]. All plasmids were based on pGEM transcription vectors.
- Figure 3 shows the translation products of pGUS, pCATGUS, pCAT2AGUS and pCAT; and,
- Figure 4 shows CAT and GUS activity in transgenic plants transformed with pCAT2AGUS.
-
- The reporter genes CAT and GUS were amplified by PCR using oligonucleotide primers such that restriction sites were created at both termini. Individual genes were cloned into pGEM transcription vectors (pCAT; pGUS) and also assembled together (pCATGUS) to produce a single open reading frame encoding the artificial polyprotein [CATGUS] (Figure 2). Coding sequences from the
FMDV 2A region were assembled in the plasmid vector pGEM 7zf(+) in such a way that a series of unique restriction sites were created throughout the sequence. TheFMDV 2A sequence was excised and inserted between the CAT and GUS genes of pCATGUS to retain a single open reading frame and form construct pCAT2AGUS (Figure 2). - Translation studies were performed in a coupled transcription/ translation (TnT) wheat germ system using T7 polymerase. Translation directed by plasmids pCAT , pGUS and pCATGUS yielded polypeptides of the expected molecular weight for CAT (25.7kDa), GUS (70.4kDa) and the polyprotein [CATGUS] (96.3kDa) respectively (Figure 3,
lanes lane 1 and represents GUS polypeptide processed from the [CAT2AGUS] polyprotein during translation. The 26kDa band migrated slightly more slowly than the product of pCAT shown inlane 4 and corresponds to the [CAT-2A] cleavage product. A third fainter band appeared at approx. 96kDa (lane 3) and co-migrated with the product of pCATGUS (lane 2). This corresponds to the entire polyprotein product of pCAT2AGUS and suggests that a small proportion of the polyprotein is not processed in the wheat germ lysate. Densitometric analysis of the distribution of radiolabel in the polypeptides inlane 3 showed that over 90% of the [CAT2AGUS] translation product was cleaved to [CAT-2A] and GUS. - The [CAT2AGUS] portion of pCAT2AGUS was excised, inserted between the 35S CaMV promoter and nos 3' terminator and cloned into a Binl9-derived plant expression vector containing a functional neomycin phosphotransferase gene. This construct was introduced into tobacco via Agrobacterium-mediated leaf disk transformation. Transformed plants were selected and rooted on kanamycin. Protein extracts were prepared from leaves of transformed plants and assayed for GUS and CAT activities. The results are shown in Figure 4. A high degree of correlation was found between the activities of the two enzymes in any given plant. Of 18 independent transformed plants, seven plants (6, 26, 28, 24, 29, 1 and 12) expressed both enzymes at relatively high levels. Four plants (2, 14, 15, 16) expressed both enzymes at low levels. The remaining plants (only three shown in Figure 4,
plants - Western blots of callus and leaf extracts were probed with anti-GUS antibodies. A major immuno-reactive product was detected at the expected molecular weight for GAS (70kDa) in plants transformed with [CAT2AGUS] but not in control plants. This confirmed that [CAT2AGUS] expressed in plant tissue is processed to [CAT2A] and GUS.
- The data presented here demonstrates that the
FMDV 2A sequence can function in a manner similar to that observed in FMDV polyprotein processing when expressed in chimeric genes in plant extracts and cells. Both in wheat germ lysates and transgenic plants, the chimeric [CAT2AGUS] polyprotein undergoes rapid, apparently autoproteolytic, cleavage to yield [CAT-2A] and GUS. -
FMDV 2A may represent an entirely novel type of protein cleavage activity. Although the mechanism of cleavage is not yet understood, its utility is apparent. Because of it's small size theFMDV 2A sequence or derivatives of it are particularly attractive candidates for use in plant polyprotein expression constructs enabling the coordinated and stoichiometric expression of multiple proteins from a single open reading frame. - In the model [CAT2AGUS] construct described above, the 20
amino acid 2A-spanning sequence which remains attached to CAT after cleavage from GUS, is sufficiently short that CAT activity is not impaired. We have also shown no impairment of activity in similar constructs where 2A is attached to the carboxy terminus of glutathione-S-transferase or T7 RNA polymerase. - The
FMDV 2A sequence inserted between protein coding sequences, allows the engineering of plant expression vectors where multiple whole proteins or protein domains can be expressed as a polyprotein and cleaved apart co-translationally with high efficiency. This may enable the rapid introduction of entire enzyme cascades into plants. - An G. 1986 Plant Physiol. 81, 86-91.
- Jones J.D.G., Gilbert D.E., Grady K.L., Jorgensen R.A. 1987 Mol.Gen.Genet. 207, p478-485.
- Nagy F., Morelli G., Fraley R.T., Rogers S.G. and Chua N.-H. 1985 EMBO J. 12, 3063-3068.
- Gidoni D., Bond-Nutter D., Brosio P., Jones J., Bedbrook J. and Dunsmuir P. 1988 Mol.Gen.Genet. 211, p.507-514.
- Peach C. and Velten J. 1991 Plant Mol.Biol. 17, p.49-60.
- Roosien, J., Belsham, G.J., Ryan, M.D., King, A.M.Q. and Vlak, J.M. (1990). J. Gen. Virol. 71, 1703-1711.
- Ryan, M.D., Belsham, G.J. and King, A.M.Q. (1989). Virology 173, 35-45.
- Ryan M.D., King A.M.Q. and Thomas G.P. (1991). J.Gen. Virol. 72, 2727-2732.
- Ryan M.D. and Drew J. 1994 EMBO J. 13, 928-933.
-
- (1) GENERAL INFORMATION:
- (i) APPLICANT: ZENECA LIMITED
HALPIN, CLAIRE
RYAN, MARTIN D - (ii) TITLE OF INVENTION: EXPRESSION OF SELF-PROCESSING POLYPROTEIN IN PLANTS
- (iii) NUMBER OF SEQUENCES: 3
- (iv) CORRESPONDENCE ADDRESS:
- (A) ADDRESSEE: ZENECA SEEDS, IP SECTION,
- (B) STREET: JEALOTTS HILL RESEARCH STATION,
- (C) CITY: WARFIELD, BRACKNELL,
- (D) STATE: BERKSHIRE,
- (E) COUNTRY: UNITED KINGDOM,
- (F) ZIP: RG12 6EY
- (v) COMPUTER READABLE FORM:
- (A) MEDIUM TYPE: Floppy disk
- (B) COMPUTER: IBM PC compatible
- (C) OPERATING SYSTEM: PC-DOS/MS-DOS
- (D) SOFTWARE: PatentIn Release #1.0, Version #1.25
- (vi) CURRENT APPLICATION DATA:
- (A) APPLICATION NUMBER:
- (B) FILING DATE:
- (C) CLASSIFICATION:
- (viii) ATTORNEY/AGENT INFORMATION:
(A) NAME: HUSKISSON, FRANK M - (ix) TELECOMMUNICATION INFORMATION:
- (A) TELEPHONE: 44 1344 414822
- (B) TELEFAX: 44 1344 413646
- (2) INFORMATION FOR SEQ ID NO:1:
- (i) SEQUENCE CHARACTERISTICS:
- (A) LENGTH: 19 amino acids
- (B) TYPE: amino acid
- (D) TOPOLOGY: linear
- (ii) MOLECULE TYPE: protein
- (xi) SEQUENCE DESCRIPTION: SEQ ID NO:1:

- (2) INFORMATION FOR SEQ ID NO:2:
- (i) SEQUENCE CHARACTERISTICS:
- (A) LENGTH: 13 amino acids
- (B) TYPE: amino acid
- (D) TOPOLOGY: linear
- (ii) MOLECULE TYPE: protein
- (xi) SEQUENCE DESCRIPTION: SEQ ID NO:2:

- (2) INFORMATION FOR SEQ ID NO:3:
- (i) SEQUENCE CHARACTERISTICS:
- (A) LENGTH: 11 amino acids
- (B) TYPE: amino acid
- (D) TOPOLOGY: linear
- (ii) MOLECULE TYPE: protein
- (xi) SEQUENCE DESCRIPTION: SEQ ID NO:3:

-
Claims (5)
- A method for the expression of multiple proteins in a transgenic plant comprising inserting into the genome of the plant a gene construct comprising a 5'-region which includes a promoter which is capable of initiating transcription of a structural gene under the control thereof, a protein encoding sequence coding for more than one protein and a 3'-terminator region which includes a polyadenylation signal, each of the said protein encoding sequences being separated from an adjacent protein encoding sequence by a DNA linker sequence which on translation autoproteolytically cleaves to give the component protein molecules.
- A method as claimed in claim 1, in which the DNA sequence which encodes the post-translation cleavage site is derived from a virus, particularly a picornavirus.
- A method as claimed in claim 1, in which the DNA sequence providing the cleavage site encodes the amino acid sequence NFDLLKLAGDVESNPGPFF.
- A gene construct for the use in the genetic modification of plants comprising in sequence, a gene promoter active in plant cells, a plurality of coding regions and a 3'-non-translated region containing a polyadenylation signal, characterised in the each of the plurality of coding regions is separated by a DNA linker sequence which on translation is autoproteolytically cleaved to give the component protein molecules.
- A gene construct as claimed in claim 4, in which the cleavage site has the amino acid sequence NFDLLKLAGDVESNPGPFF.
Applications Claiming Priority (3)
| Application Number | Priority Date | Filing Date | Title |
|---|---|---|---|
| GB9326271 | 1993-12-23 | ||
| GB939326271A GB9326271D0 (en) | 1993-12-23 | 1993-12-23 | Expression of self-processing polyprotein in transgenic plants |
| PCT/GB1994/002765 WO1995017514A1 (en) | 1993-12-23 | 1994-12-19 | Expression of self-processing polyproteins in transgenic plants |
Publications (2)
| Publication Number | Publication Date |
|---|---|
| EP0736099A1 EP0736099A1 (en) | 1996-10-09 |
| EP0736099B1 true EP0736099B1 (en) | 2001-10-24 |
Family
ID=10747081
Family Applications (1)
| Application Number | Title | Priority Date | Filing Date |
|---|---|---|---|
| EP95903855A Expired - Lifetime EP0736099B1 (en) | 1993-12-23 | 1994-12-19 | Expression of self-processing polyproteins in transgenic plants |
Country Status (9)
| Country | Link |
|---|---|
| US (1) | US5846767A (en) |
| EP (1) | EP0736099B1 (en) |
| JP (1) | JPH09506773A (en) |
| AT (1) | ATE207541T1 (en) |
| AU (1) | AU696643B2 (en) |
| CA (1) | CA2176209A1 (en) |
| DE (1) | DE69428804T2 (en) |
| GB (1) | GB9326271D0 (en) |
| WO (1) | WO1995017514A1 (en) |
Cited By (2)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US8945876B2 (en) | 2011-11-23 | 2015-02-03 | University Of Hawaii | Auto-processing domains for polypeptide expression |
| US10011847B2 (en) | 2013-05-20 | 2018-07-03 | 3P Biopharmaceuticals, S.L. | Alphaviral vectors and cell lines for producing recombinant proteins |
Families Citing this family (24)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US5965789A (en) * | 1991-01-11 | 1999-10-12 | American Red Cross | Engineering protein posttranslational modification by PACE/furin in transgenic non-human mammals |
| US5912167A (en) * | 1995-06-06 | 1999-06-15 | Wisconsin Alumni Research Foundation | Autocatalytic cleavage site and use thereof in a protein expression vector |
| AU5434099A (en) * | 1998-08-18 | 2000-03-14 | Syngenta Limited | Genetic method for the expression of polyproteins in plants |
| US6053454A (en) * | 1998-09-04 | 2000-04-25 | Hughes Electronics Corporation | Modular spacecraft payload support structure |
| US6921634B2 (en) * | 1999-12-23 | 2005-07-26 | Board Of Regents, The University Of Texas System | Replication competent hepatitus C virus and methods of use |
| ES2340915T3 (en) * | 2000-11-17 | 2010-06-11 | Metabolix, Inc. | PRODUCTION OF AVERAGE CHAIN LENGTH POLYHYDROXIALCANOATES BY ROADS OF BIOSYNTHESIS OF FATTY ACIDS. |
| EP1356063B8 (en) * | 2001-01-30 | 2005-08-10 | Wisconsin Alumni Research Foundation | Expression of multiple proteins in transgenic plants |
| US20050136035A1 (en) * | 2003-06-03 | 2005-06-23 | Derek Ko | Cell specific replication-competent viral vectors comprising a self processing peptide cleavage site |
| WO2005017149A1 (en) * | 2003-06-03 | 2005-02-24 | Cell Genesys, Inc. | Compositions and methods for enhanced expression of recombinant polypeptides from a single vector using a peptide cleavage site |
| US7485291B2 (en) * | 2003-06-03 | 2009-02-03 | Cell Genesys, Inc. | Compositions and methods for generating multiple polypeptides from a single vector using a virus derived peptide cleavage site, and uses thereof |
| WO2005053516A2 (en) * | 2003-12-01 | 2005-06-16 | Boards Of Regents, The University Of Texas System | Replication competent hepatitis c virus and methods of use |
| EP1765846A4 (en) * | 2004-07-13 | 2010-02-17 | Cell Genesys Inc | Aav vector compositions and methods for enhanced expression of immunoglobulins using the same |
| US7632509B2 (en) * | 2005-07-19 | 2009-12-15 | Biosante Pharmaceuticals, Inc. | Methods to express recombinant proteins from lentiviral vectors |
| CN101595228A (en) | 2005-07-21 | 2009-12-02 | 艾博特公司 | Multi-gene expression including SORF constructs and methods of using polyproteins, precursor proteins, and proteolysis |
| WO2007123737A2 (en) | 2006-03-30 | 2007-11-01 | University Of California | Methods and compositions for localized secretion of anti-ctla-4 antibodies |
| US7919079B2 (en) * | 2006-03-31 | 2011-04-05 | Biosante Pharmaceuticals, Inc. | Cancer immunotherapy compositions and methods of use |
| US20070292922A1 (en) * | 2006-03-31 | 2007-12-20 | Cell Genesys, Inc. | Regulated expression of recombinant proteins from adeno-associated viral vectors |
| WO2008065225A2 (en) | 2006-11-28 | 2008-06-05 | Proyecto De Biomedicina Cima, S.L. | Viral vector and uses thereof |
| US8609936B2 (en) | 2007-04-27 | 2013-12-17 | Monsanto Technology Llc | Hemipteran-and coleopteran active toxin proteins from Bacillus thuringiensis |
| JP2013509188A (en) * | 2009-10-30 | 2013-03-14 | アボット・ラボラトリーズ | SORF constructs and multiple gene expression |
| WO2011064437A2 (en) | 2009-11-26 | 2011-06-03 | Proyecto De Biomedicina Cima, S.L. | Viral vectors and methods used in the preparation of gdnf |
| WO2012001196A2 (en) | 2010-06-28 | 2012-01-05 | Proyecto De Biomedicina Cima, S.L. | Alphaviral vectors and the uses thereof for heterologous gene expression |
| EP2407534A1 (en) | 2010-07-14 | 2012-01-18 | Neo Virnatech, S.L. | Methods and reagents for obtaining transcriptionally active virus-like particles and recombinant virions |
| WO2019200013A1 (en) | 2018-04-11 | 2019-10-17 | Cancer Targeting Systems, Inc. | Therapeutic constructs for treating cancer |
Family Cites Families (1)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US5162601A (en) * | 1989-11-22 | 1992-11-10 | The Upjohn Company | Plant potyvirus expression vector with a gene for protease |
-
1993
- 1993-12-23 GB GB939326271A patent/GB9326271D0/en active Pending
-
1994
- 1994-12-19 CA CA002176209A patent/CA2176209A1/en not_active Abandoned
- 1994-12-19 US US08/646,293 patent/US5846767A/en not_active Expired - Fee Related
- 1994-12-19 JP JP7517258A patent/JPH09506773A/en active Pending
- 1994-12-19 AT AT95903855T patent/ATE207541T1/en not_active IP Right Cessation
- 1994-12-19 EP EP95903855A patent/EP0736099B1/en not_active Expired - Lifetime
- 1994-12-19 DE DE69428804T patent/DE69428804T2/en not_active Expired - Fee Related
- 1994-12-19 WO PCT/GB1994/002765 patent/WO1995017514A1/en not_active Ceased
- 1994-12-19 AU AU12762/95A patent/AU696643B2/en not_active Ceased
Cited By (2)
| Publication number | Priority date | Publication date | Assignee | Title |
|---|---|---|---|---|
| US8945876B2 (en) | 2011-11-23 | 2015-02-03 | University Of Hawaii | Auto-processing domains for polypeptide expression |
| US10011847B2 (en) | 2013-05-20 | 2018-07-03 | 3P Biopharmaceuticals, S.L. | Alphaviral vectors and cell lines for producing recombinant proteins |
Also Published As
| Publication number | Publication date |
|---|---|
| WO1995017514A1 (en) | 1995-06-29 |
| DE69428804D1 (en) | 2001-11-29 |
| GB9326271D0 (en) | 1994-02-23 |
| US5846767A (en) | 1998-12-08 |
| DE69428804T2 (en) | 2002-04-25 |
| AU696643B2 (en) | 1998-09-17 |
| ATE207541T1 (en) | 2001-11-15 |
| EP0736099A1 (en) | 1996-10-09 |
| CA2176209A1 (en) | 1995-06-29 |
| AU1276295A (en) | 1995-07-10 |
| JPH09506773A (en) | 1997-07-08 |
Similar Documents
| Publication | Publication Date | Title |
|---|---|---|
| AU696643B2 (en) | Expression of self-processing polyproteins in transgenic plants | |
| US5162601A (en) | Plant potyvirus expression vector with a gene for protease | |
| AU634168B2 (en) | Potyvirus coat protein genes and plants transformed therewith | |
| Verchot et al. | The 35-kDa protein from the N-terminus of the potyviral polyprotein functions as a third virus-encoded proteinase | |
| Schaad et al. | Analysis of the VPg-proteinase (NIa) encoded by tobacco etch potyvirus: effects of mutations on subcellular transport, proteolytic processing, and genome amplification | |
| Carrington et al. | Expression of potyviral polyproteins in transgenic plants reveals three proteolytic activities required for complete processing. | |
| Lee et al. | The complete sequence (22 kilobases) of murine coronavirus gene 1 encoding the putative proteases and RNA polymerase | |
| US5491076A (en) | Expression of foreign genes using a replicating polyprotein producing virus vector | |
| Basso et al. | Evidence for an internal ribosome entry site within the 5′ non-translated region of turnip mosaic potyvirus RNA | |
| US5846795A (en) | RNA transformation vector | |
| Sasaki et al. | An insect picorna-like virus, Plautia stali intestine virus, has genes of capsid proteins in the 3′ part of the genome | |
| WO1990012107A1 (en) | Recombinant expression system based on satellite tobacco mosaic virus | |
| CA2278523C (en) | Rna binding protein and binding site useful for expression of recombinant molecules | |
| JP2002176995A (en) | Synthetic genes for insecticidal crystal proteins | |
| AU693770B2 (en) | RNA packaging system | |
| Hughes et al. | Identification of the murine coronavirus p28 cleavage site | |
| Ma et al. | Expressing multiple genes in a single open reading frame with the 2A region of foot-and-mouth disease virus as a linker | |
| Marcos et al. | In vitro characterization of a cassette to accumulate multiple proteins through synthesis of a self-processing polypeptide | |
| CA2078134A1 (en) | Transformation of plants with non-structural plant virus gene sequences | |
| EP0786003A1 (en) | Insect viruses and their uses in protecting plants | |
| WO1987003619A1 (en) | PROCESS FOR ENHANCING TRANSLATIONAL EFFICIENCY OF EUKARYOTIC mRNA | |
| WO1995033834B1 (en) | Lag1: a gene for increasing the longevity of eukaryotes | |
| Cao et al. | Genetic variation of the poliovirus genome with two VPg coding units. | |
| WO1995021249A1 (en) | A cassette to accumulate multiple proteins through synthesis of a self-processing polypeptide | |
| US20060127364A1 (en) | Insect viruses and their uses in protecting plants |
Legal Events
| Date | Code | Title | Description |
|---|---|---|---|
| PUAI | Public reference made under article 153(3) epc to a published international application that has entered the european phase |
Free format text: ORIGINAL CODE: 0009012 |
|
| 17P | Request for examination filed |
Effective date: 19960723 |
|
| AK | Designated contracting states |
Kind code of ref document: A1 Designated state(s): AT BE CH DE DK ES FR GB GR IE IT LI LU MC NL PT SE |
|
| 17Q | First examination report despatched |
Effective date: 19991228 |
|
| GRAG | Despatch of communication of intention to grant |
Free format text: ORIGINAL CODE: EPIDOS AGRA |
|
| RAP1 | Party data changed (applicant data changed or rights of an application transferred) |
Owner name: SYNGENTA LIMITED |
|
| GRAG | Despatch of communication of intention to grant |
Free format text: ORIGINAL CODE: EPIDOS AGRA |
|
| GRAH | Despatch of communication of intention to grant a patent |
Free format text: ORIGINAL CODE: EPIDOS IGRA |
|
| GRAH | Despatch of communication of intention to grant a patent |
Free format text: ORIGINAL CODE: EPIDOS IGRA |
|
| GRAA | (expected) grant |
Free format text: ORIGINAL CODE: 0009210 |
|
| AK | Designated contracting states |
Kind code of ref document: B1 Designated state(s): AT BE CH DE DK ES FR GB GR IE IT LI LU MC NL PT SE |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: IT Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRE;WARNING: LAPSES OF ITALIAN PATENTS WITH EFFECTIVE DATE BEFORE 2007 MAY HAVE OCCURRED AT ANY TIME BEFORE 2007. THE CORRECT EFFECTIVE DATE MAY BE DIFFERENT FROM THE ONE RECORDED.SCRIBED TIME-LIMIT Effective date: 20011024 Ref country code: GR Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20011024 Ref country code: BE Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20011024 Ref country code: AT Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20011024 |
|
| REF | Corresponds to: |
Ref document number: 207541 Country of ref document: AT Date of ref document: 20011115 Kind code of ref document: T |
|
| REG | Reference to a national code |
Ref country code: CH Ref legal event code: EP |
|
| REG | Reference to a national code |
Ref country code: IE Ref legal event code: FG4D |
|
| REG | Reference to a national code |
Ref country code: CH Ref legal event code: NV Representative=s name: BOVARD AG PATENTANWAELTE |
|
| REF | Corresponds to: |
Ref document number: 69428804 Country of ref document: DE Date of ref document: 20011129 |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: MC Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20011219 Ref country code: LU Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20011219 Ref country code: IE Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20011219 |
|
| REG | Reference to a national code |
Ref country code: GB Ref legal event code: IF02 |
|
| ET | Fr: translation filed | ||
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: SE Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20020124 Ref country code: PT Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20020124 Ref country code: DK Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20020124 |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: ES Free format text: LAPSE BECAUSE OF FAILURE TO SUBMIT A TRANSLATION OF THE DESCRIPTION OR TO PAY THE FEE WITHIN THE PRESCRIBED TIME-LIMIT Effective date: 20020430 |
|
| PLBE | No opposition filed within time limit |
Free format text: ORIGINAL CODE: 0009261 |
|
| STAA | Information on the status of an ep patent application or granted ep patent |
Free format text: STATUS: NO OPPOSITION FILED WITHIN TIME LIMIT |
|
| RAP2 | Party data changed (patent owner data changed or rights of a patent transferred) |
Owner name: SYNGENTA LIMITED |
|
| REG | Reference to a national code |
Ref country code: IE Ref legal event code: MM4A |
|
| 26N | No opposition filed | ||
| NLT2 | Nl: modifications (of names), taken from the european patent patent bulletin |
Owner name: SYNGENTA LIMITED |
|
| REG | Reference to a national code |
Ref country code: CH Ref legal event code: PFA Owner name: SYNGENTA LIMITED SYNGENTA EUROPEAN REGIONAL CENTR Free format text: SYNGENTA LIMITED#FERNHURST#HASLEMERE, SURREY GU27 3JE (GB) -TRANSFER TO- SYNGENTA LIMITED SYNGENTA EUROPEAN REGIONAL CENTRE#PRIESTLEY ROAD, SURREY RESEARCH PARK,#GUILDFORD, SURREY GU2 7YH (GB) |
|
| PGFP | Annual fee paid to national office [announced via postgrant information from national office to epo] |
Ref country code: NL Payment date: 20041205 Year of fee payment: 11 |
|
| PGFP | Annual fee paid to national office [announced via postgrant information from national office to epo] |
Ref country code: FR Payment date: 20041208 Year of fee payment: 11 |
|
| PGFP | Annual fee paid to national office [announced via postgrant information from national office to epo] |
Ref country code: CH Payment date: 20041215 Year of fee payment: 11 |
|
| PGFP | Annual fee paid to national office [announced via postgrant information from national office to epo] |
Ref country code: DE Payment date: 20041216 Year of fee payment: 11 |
|
| REG | Reference to a national code |
Ref country code: GB Ref legal event code: 732E |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: LI Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20051231 Ref country code: CH Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20051231 |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: NL Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20060701 Ref country code: DE Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20060701 |
|
| REG | Reference to a national code |
Ref country code: CH Ref legal event code: PL |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: FR Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20060831 |
|
| NLV4 | Nl: lapsed or anulled due to non-payment of the annual fee |
Effective date: 20060701 |
|
| REG | Reference to a national code |
Ref country code: FR Ref legal event code: ST Effective date: 20060831 |
|
| PGFP | Annual fee paid to national office [announced via postgrant information from national office to epo] |
Ref country code: GB Payment date: 20091216 Year of fee payment: 16 |
|
| GBPC | Gb: european patent ceased through non-payment of renewal fee |
Effective date: 20101219 |
|
| PG25 | Lapsed in a contracting state [announced via postgrant information from national office to epo] |
Ref country code: GB Free format text: LAPSE BECAUSE OF NON-PAYMENT OF DUE FEES Effective date: 20101219 |